Organismal Biology · Unit 2: Control and constancy
Metabolic Rate and Body Temperature
What sets an animal's body temperature: the heat it makes, the heat it loses, or a controller deciding between them? This lesson defines metabolic rate and the conditions it is measured under, contrasts endotherms with ectotherms using a desert lizard, a laboratory mouse and a fish that warms itself, and follows heat out of the body by four routes. Afterwards you can read a thermoneutral-zone plot, calculate the extra energy an endotherm spends in colder air, and explain why fever, torpor and hibernation are regulated changes rather than failures.
Watch first Heat Made, Heat Lost, Set Point · 3:05
A desert iguana basking on a rock can end up warmer than you are, and a hibernating American black bear stays at roughly 30 to 36 degrees C while running on a quarter of its basal energy use. So “cold-blooded” and “warm-blooded” tell you little. What does an animal’s temperature depend on: the heat it makes, the heat it loses, or a controller?
Metabolic rate: how fast an animal spends energy
Metabolic rate is the energy an animal uses per unit time, in watts (joules per second) or kilojoules per day. Nearly all of that energy ends up as heat.
In indirect calorimetry, or respirometry, an animal sits in a chamber with a known airflow, and you record the oxygen it takes up and the carbon dioxide it gives off. Each litre of oxygen consumed corresponds to roughly 20 kJ, depending on the fuel burned (see integration of metabolism).
A rate means little without its conditions.
- Basal metabolic rate (BMR) is measured in an endotherm that is awake, resting, postabsorptive (not digesting a meal) and within its thermoneutral zone, the range of air temperatures over which it spends no extra energy on heating or cooling.
- Standard metabolic rate (SMR) is the equivalent for an ectotherm: resting, postabsorptive, and at a stated temperature, because its rate changes with temperature. In threespine sticklebacks acclimated to 5, 12 or 20 degrees C for 7 to 21 weeks, SMR rose with acclimation temperature.
- Daily energy expenditure is everything over 24 hours: activity, digestion, heating, growth.
Exercise raises daily expenditure; it does not raise BMR, which by definition is measured at rest. In single-housed male laboratory mice (Fischer, Cannon and Nedergaard, 2018), mean 24-hour expenditure was 3.1 times the thermoneutral resting rate in mice kept at 21 degrees C.
Across mammals and birds, whole-body BMR rises with mass to roughly the 3/4 power (Kleiber’s relation), so a gram of mouse spends far more than a gram of elephant. That exponent is a fitted value, some analyses find nearer 2/3, and its cause is unsettled; see size and scaling.
A lizard, a mouse and a fish that warms itself
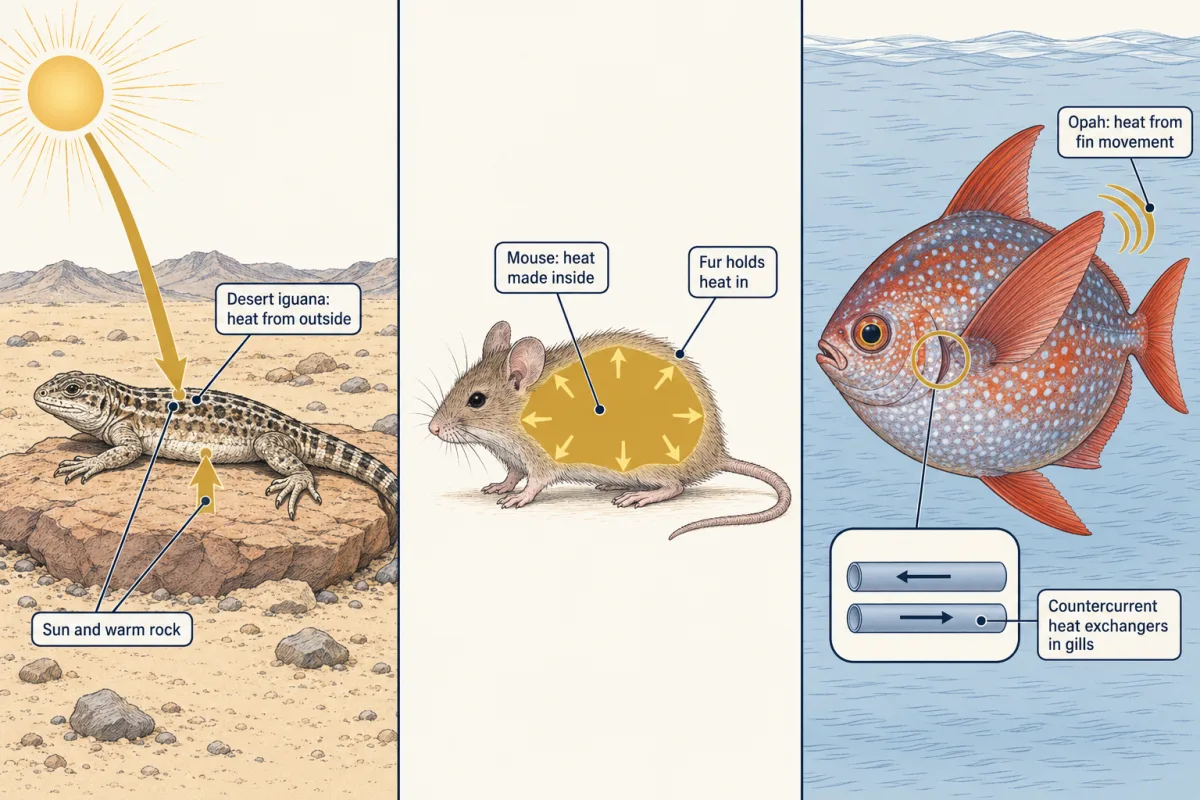
An endotherm, such as a mammal or bird, warms itself mainly with heat from its own metabolism, held in by insulation. An ectotherm takes its body temperature mainly from outside: sun, warm rock, water. Most fish, amphibians, reptiles and invertebrates are ectotherms. A homeotherm holds a nearly constant body temperature, and a heterotherm lets it vary widely. Where the heat comes from and how constant the temperature is are separate questions: a deep-sea fish in steady cold is a nearly constant ectotherm, and a hibernating ground squirrel a heterothermic endotherm.
The desert iguana, Dipsosaurus dorsalis, is an ectotherm of the deserts of the southwestern United States and northwestern Mexico. It regulates its temperature by behaviour, shuttling between sun and shade or retreating into a burrow, and through the active day it can hold a body temperature near or above 37 degrees C. Ectotherm names the heat source, not a cold animal.
The laboratory mouse, Mus musculus, is a small endotherm that loses heat fast relative to its mass, so below its thermoneutral zone its expenditure rises steeply as the air cools. Škop and colleagues (2020), recording metabolic rate and body temperature together, placed the mouse’s thermoneutral point near 29 degrees C in the light phase and 33 degrees C in the dark, and found no range of air temperature where both stayed constant. Animal rooms near 20 to 22 degrees C are therefore cool for a mouse.
The opah, Lampris guttatus, shows that not every fish is an ectotherm. Tunas and lamnid sharks keep some muscles warm, and in 2015 Nicholas Wegner and colleagues reported that the opah, a disc-shaped ocean fish, warms its body with heat from continuous movement of its pectoral fins and limits heat loss with countercurrent heat exchangers in its gills. In most fish, blood leaves the gills at water temperature.
Some insects are partly endothermic too: bumblebees and many moths warm their flight muscles before take-off by a kind of shivering.
Four routes for heat, and the dials that adjust them
Heat moves by four routes.
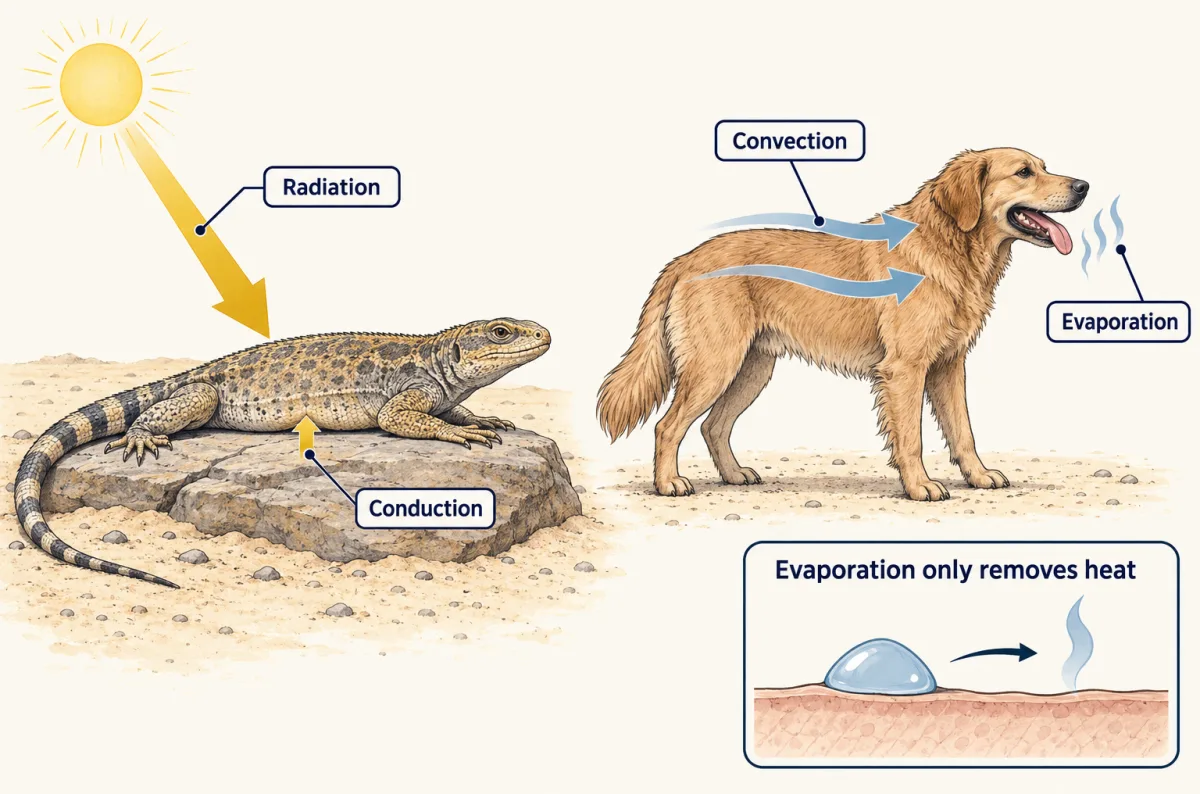
- Radiation: emission and absorption of electromagnetic energy, as when a lizard absorbs sunlight.
- Conduction: transfer between surfaces in direct contact, as from a warm belly into cold rock.
- Convection: transfer by moving air or water, as wind carries heat from skin warmer than the air.
- Evaporation: water turning to vapour takes heat with it, as in sweating in humans and horses or panting in dogs and many birds.
The first three run either way, depending on which side is warmer. Evaporation only removes heat, and it costs water (see osmoregulation). Each route’s share depends on species, size, posture and weather.
Animals adjust these routes with a few dials.
- Insulation. Fur and feathers trap still air; many marine mammals rely on blubber.
- Skin blood flow. Narrowing the small arteries to the skin (vasoconstriction) keeps warm blood in the core; widening them (vasodilation) delivers heat to the surface. (See blood vessels, blood and lymph.)
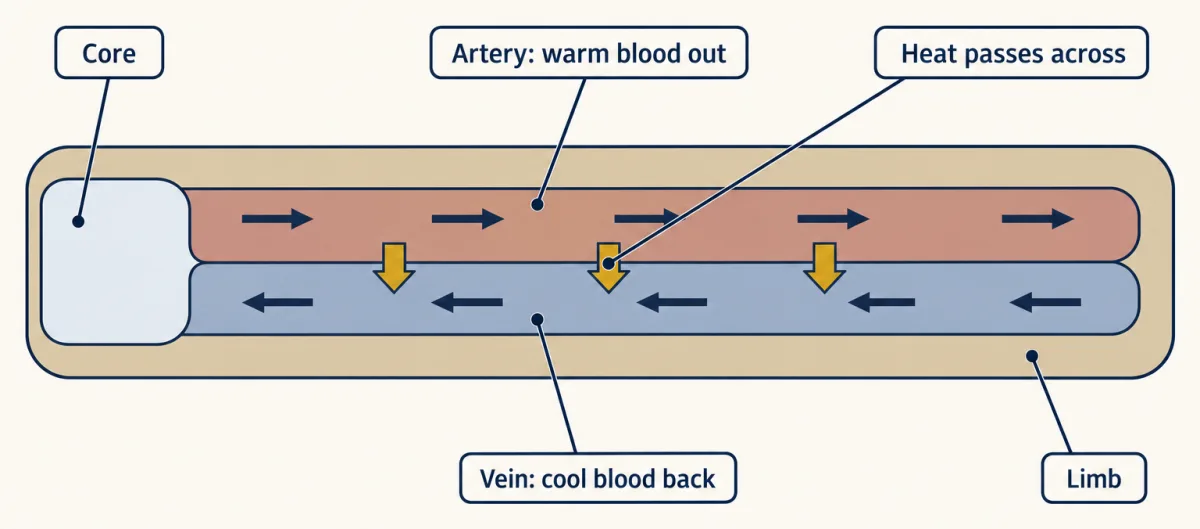
- Countercurrent exchange. When an artery carrying warm blood out to a limb runs alongside the vein bringing cool blood back, heat passes across, so much of it returns to the core. The legs of many birds and the flippers of whales and seals work this way, as do the opah’s gills.
- Evaporative cooling, by sweating, panting or licking.
- Behaviour: basking, seeking shade, huddling, burrowing.
Endotherms can also turn up heat production. Shivering is rapid, unsynchronized muscle contraction that releases heat. Many mammals also have brown adipose tissue, whose mitochondria carry the protein UCP1, which lets protons leak back across the inner membrane so food energy becomes heat instead of ATP (see the proton-motive force). The control signals come from the hypothalamus.
Now plot an endotherm’s resting metabolic rate against air temperature. Within the thermoneutral zone the line is flat, at BMR. Below the lower critical temperature it climbs. Above the upper critical temperature it rises again, as panting and sweating take work. The steepness of the cold limb (the size of its slope) equals the animal’s thermal conductance, how readily heat leaks out per degree of difference. In 1950 Per Scholander, Laurence Irving and colleagues found that thick-furred arctic mammals stay on the flat part into much colder air than tropical ones, mainly because their insulation lowers conductance.
Worked problem. The numbers here are invented for practice. A small endotherm holds its body temperature at 37 degrees C with a constant conductance C = 0.020 W per K. Assume steady state (no heat stored), no external work, and air temperatures below its lower critical temperature, so heat production equals heat loss:
heat production (W) = C (W per K) x (body temperature - air temperature) (K)
- At 27 degrees C the difference is 10 K. Heat production = 0.020 W per K x 10 K = 0.20 W.
- At 17 degrees C the difference is 20 K. Heat production = 0.020 W per K x 20 K = 0.40 W.
- Extra power: 0.40 W - 0.20 W = 0.20 W. Check: 0.020 W per K x (27 - 17) K = 0.20 W.
- Extra energy in a day: 0.20 J per s x 86,400 s = 17,280 J, or 17.28 kJ.
- Assume fat yields about 39 kJ per g. Then 17.28 kJ / 39 kJ per g = about 0.44 g of fat per day.
The cost doubled only because these numbers double the gradient with C fixed; 10 degrees of cooling does not generally double metabolism. Fluff the fur so C falls to 0.010 W per K, and the cost at 17 degrees C drops back to 0.20 W.
- Heat production at air 1
- Heat production at air 2
- Extra power (air 2 minus air 1)
- Extra energy per day
- Fat for that energy, assuming fat yields about 39 kJ per g
In this sketch (invented numbers for a small endotherm): steady state, no heat stored, no external work, constant conductance, body held at 37 °C, air below the lower critical temperature.
Below the lower critical temperature the size of the slope (steepness) of the line is the conductance; with C fixed, a bigger gap between body and air means more heat to make.
Fever, torpor and hibernation are regulated
A set point is the value a control system defends, and in fever, torpor and hibernation the defended value shifts (tissues, organs and homeostasis introduced set points).
Fever is regulation of body temperature at a raised level. In mammals, signals from an infection reach the brain’s temperature-control region; in mice given bacterial lipopolysaccharide into a vein, prostaglandin made by the cells lining brain blood vessels supplied the fever signal. Innate immunity follows the immune side. The body then conserves heat and shivers until it reaches the new level.
Ectotherms have fever too, by behaviour: infected desert iguanas offered a choice of temperatures settled about 2 degrees C warmer. Does that help? Matthew Kluger, D. H. Ringler and M. R. Anver tested this in 1975. They injected desert iguanas with live bacteria and held each lizard at one constant air temperature, 34, 36, 38, 40 or 42 degrees C, so it could not choose. If fever were a harmless side effect, survival should not depend on temperature. Instead survival was greater at the higher temperatures than at the lowest. That rules in a survival benefit of raised temperature in this lizard with this infection, not in mammals or other infections, and it does not show what the warmth changed in the host or the bacteria.
Torpor is a controlled drop in metabolic rate and body temperature in a bird or mammal. Daily torpor conventionally lasts under 24 hours; fasted laboratory mice housed at 22 degrees C enter it, cooling for hours and then rewarming. Hibernation is a series of torpor bouts, each lasting days to several weeks, typically broken by periodic arousals that are costly in energy. Many small hibernators, such as ground squirrels, let body temperature fall to near freezing.
Torpor is controlled. In mice, Siniša Hrvatin and colleagues (2020) found that reactivating neurons in the hypothalamic preoptic area brought on key features of torpor in mice that were not food-restricted, and that inhibiting an identified group of them disrupted natural torpor. In black bears, metabolism falls further than cooling explains.
Design problem
Is hibernation just cooling? Use illustrative numbers in the pattern of Tøien and colleagues (2011): a black bear’s metabolic rate falls to 25% of basal while its body temperature falls from 37 to 33 degrees C. Assume a Q10 (the factor by which a rate changes per 10 degree C change in temperature) of 2.5. How much of the fall could cooling explain, and what measurement would separate cooling from active suppression?
One way to do it
Passive cooling predicts:
predicted fraction of basal = Q10 ^ ((T - T0) / 10) = 2.5 ^ (-4 / 10) = 2.5 ^ (-0.4)
ln 2.5 = 0.916; times -0.4 gives -0.367; e ^ (-0.367) = 0.69. Cooling alone predicts 69% of basal. The bear is at 25%, so a further factor of 0.25 / 0.69 = 0.36 is left unexplained by temperature: most of the suppression is something other than cooling.
To separate the two, record oxygen consumption and body temperature together, continuously, through hibernation and emergence. If metabolism simply followed temperature, it would recover when temperature does. In the real bears it stayed low for up to three weeks after body temperature had returned to normal and they had emerged, which separates the two in time.
The Q10 of 2.5 is an assumption; there is no universal Q10. And a bear’s answer does not transfer to a ground squirrel that cools near 0 degrees C, where the much larger temperature fall may account for more of the drop.
How we measure it
Indirect calorimetry (respirometry)
Place the animal in a chamber with a known airflow and measure how much oxygen it takes up and how much carbon dioxide it gives off. Oxygen use converts to energy use, about 20 kJ per litre of oxygen depending on the fuel, so this gives metabolic rate without measuring heat directly.
Implanted temperature telemetry
Implant a small transmitter that reports internal body temperature by radio while the animal moves freely. Recorded at the same time as calorimetry, it shows whether metabolism and body temperature change together or apart, the evidence behind the mouse thermoneutral-point and bear hibernation studies.
Holding infected animals at fixed temperatures
Infect animals in the same way, then hold groups at different constant temperatures so they cannot choose their own, and compare survival. It tests whether a raised temperature changes the outcome, though by itself it does not show which process in host or microbe changed.
Whole-body thermal conductance from calorimetry
Divide an endotherm's measured heat production by the difference between its body and air temperatures, below its thermoneutral zone. The result, in watts per kelvin, is how readily heat leaks out, and it lets you compare insulation across animals or predict the cost of colder air.
Finish line
Test yourself
8 questions
Practice and MCAT-style, with explained answers.
Next · Lesson 10
Circulation and the Heart
An adult human holds about 5 litres of blood, yet at rest each side of the heart pumps about that much every minute. Where does it all go?
Continue →