Organismal Biology · Unit 6: How plants work
Plant Hormones and Responses
A plant has no nervous system and no endocrine glands, yet its shoot bends toward light, its root turns down, and it flowers in the right season. This lesson names the main plant hormones with one effect and one organism each, follows the coleoptile experiments of the Darwins, Boysen-Jensen and Went to the idea that auxin moves sideways, explains phytochrome and night length, and introduces the defence signals jasmonate and salicylic acid. Afterwards you can read a curvature bioassay and interpret a red and far-red light experiment.
Watch first Auxin Moves Sideways, and the Shoot Bends · 2:58
Light an oat seedling from one side and its shoot bends toward the lamp. The part that bends is below the tip, where the light is mainly sensed. What carries the message between them?
The answer is a chemical signal, a hormone. This lesson names the main plant hormones, follows the experiments that tracked down the first one, and shows how plants use hormones and light-sensing pigments to bend, flower and defend themselves.
Seven hormones, many effects
A hormone is a chemical made in small amounts that changes what cells do, in the cell that made it or in cells elsewhere in the body. Vertebrates make most of theirs in glands and carry them in blood (the endocrine system). Plants have no endocrine glands: many kinds of plant cell make hormones, and the response is often a change in growth. The main ones, each with one effect and the organism it was shown in:
- Auxin (the main natural form is indole-3-acetic acid, IAA) speeds elongation of shoot cells, drives tropisms, and maintains apical dominance, the suppression of side buds by the growing shoot tip. In Arabidopsis thaliana it promotes growth on the shaded side of the hypocotyl, the seedling stem below the seed leaves.
- Cytokinins promote cell division. In transgenic tobacco that made extra cytokinin in ageing leaves, leaf senescence, the programmed yellowing and death of a leaf, was delayed.
- Gibberellins promote stem elongation and seed germination. In isolated aleurone layers (the living outer layer of a cereal grain’s food store) of Himalaya barley, gibberellic acid increased synthesis of alpha-amylase, a starch-digesting enzyme, after a lag of 6 to 8 hours.
- Abscisic acid (ABA) induces stomatal closure in Arabidopsis (plant transport has the guard cells) and maintains dormancy, a state of arrested growth in seeds and buds.
- Ethylene, a gas, promotes fruit ripening. Tomatoes engineered to make little ethylene failed to ripen normally, and supplied ethylene restored ripening.
- Brassinosteroids, steroid hormones, promote cell elongation. Supplied brassinosteroids could make up for the short, poorly elongated cells of several Arabidopsis mutants.
- Jasmonates signal defence against plant-eating animals, and salicylic acid against some pathogens (end of the lesson).
Inside cells, auxin binds a receptor that triggers destruction of repressor proteins (ubiquitin and proteolysis; receptor logic is in the receptor field guide). Hold on to one point: the same hormone can act differently in different organs. Auxin speeds elongation in shoots and slows it in roots.
Bending toward light: the Darwins, Boysen-Jensen and Went
A tropism is growth toward or away from a one-sided stimulus. Phototropism is directional growth in response to light. The classic experiments used grass coleoptiles, the sheath that covers the first leaf of a grass seedling as it pushes up through the soil.
Charles Darwin, with his son Francis credited for assistance, described the first set in The Power of Movement in Plants (1880). They lit seedlings of canary grass, Phalaris canariensis, from one side. Opaque caps over the tips greatly reduced bending, even though the lower part, where the curve forms, was still lit. Transparent glass tubes over the tips did not stop bending. Light is sensed mainly near the tip, and something passes down to where bending happens.
Peter Boysen-Jensen, working with oat (Avena sativa) coleoptiles in reports from 1910 to 1913, cut off tips and set them back in place. The coleoptile still bent below the cut when its tip was lit from one side, so the influence crossed a wound. He then slipped mica, a mineral sheet that dissolved chemicals cannot cross, into a cut on one side below the tip. Mica on the lit side left bending intact. Mica on the shaded side blocked it. The signal runs down the shaded side.
Frits Went, working on oat coleoptiles at Utrecht and publishing in 1928, took the signal out of the plant. He stood cut tips of dark-grown coleoptiles on small blocks of agar, removed the tips, and set a block on one side of a decapitated coleoptile in the dark. If the tip acted only through living tissue, the block should do nothing. The coleoptile curved away from the block, and plain agar caused no curve. A substance from the tips had entered the agar and sped elongation beneath it. The angle could be measured, making a bioassay: a measurement of a chemical through the response of living tissue. Went measured growth activity, not the chemical; IAA was identified later by others.
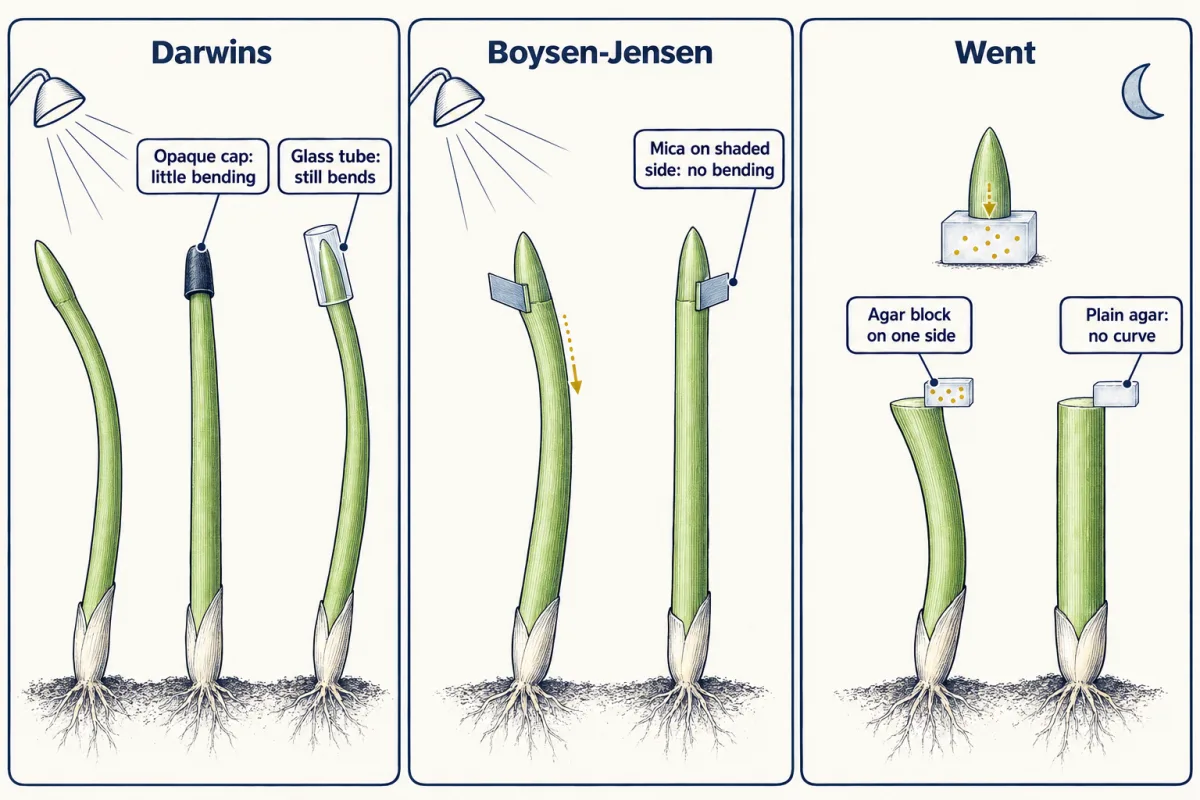
Why does the shaded side get more? The Cholodny-Went hypothesis says that light from one side moves auxin sideways toward the shaded flank, which then elongates faster, so the shoot bends toward the light. In Arabidopsis hypocotyls, light changes the position in the cell membrane of PIN3, a carrier that exports auxin from cells. PIN carriers sit on one face of a cell, so repositioning them steers auxin. The light itself is detected by a blue-light receptor first studied as NPH1, now called phototropin.
Worked problem: reading a curvature bioassay
These numbers are illustrative. Assume all agar blocks are the same size and collect for the same time, no auxin is lost, and curvature is proportional to auxin concentration in this range.
auxin concentration (mg per L) = curvature (degrees) / 200 degrees per mg per L
- Calibrate. Standard blocks with 0.02, 0.04 and 0.08 mg per L of auxin give 4, 8 and 16 degrees. In each, curvature divided by concentration is 200 degrees per mg per L.
- Split tips. Tips lit from one side are divided by a barrier, each half draining into its own block. The lit-half block gives 6 degrees: 6 / 200 = 0.03 mg per L. The shaded-half block gives 12 degrees: 12 / 200 = 0.06 mg per L.
- Shares. Total = 0.03 + 0.06 = 0.09 mg per L. Shaded share = 0.06 / 0.09 = 67%; lit share = 33%. The ratio is 2 to 1.
- Dark control. A block from whole tips kept in the dark gives 18 degrees: 18 / 200 = 0.09 mg per L, the same total.
- Block on the coleoptile
- Cursor reading
- Shares of the split tip
- Split total against dark total
- Hypothesis overlay
Rule to keep: auxin concentration (mg per L) = curvature (degrees) / 200 degrees per mg per L. In this sketch: illustrative numbers in the linear range, not data from a real experiment; equal block size and collection time; no auxin lost; the picture is a sketch of the logic, not to scale.
Light did not destroy auxin on the lit side, or the total would have fallen. It moved auxin to the shaded side, as the Cholodny-Went idea predicts. Real split-tip experiments exist; these numbers are not theirs.
Up and down: gravitropism in roots and shoots
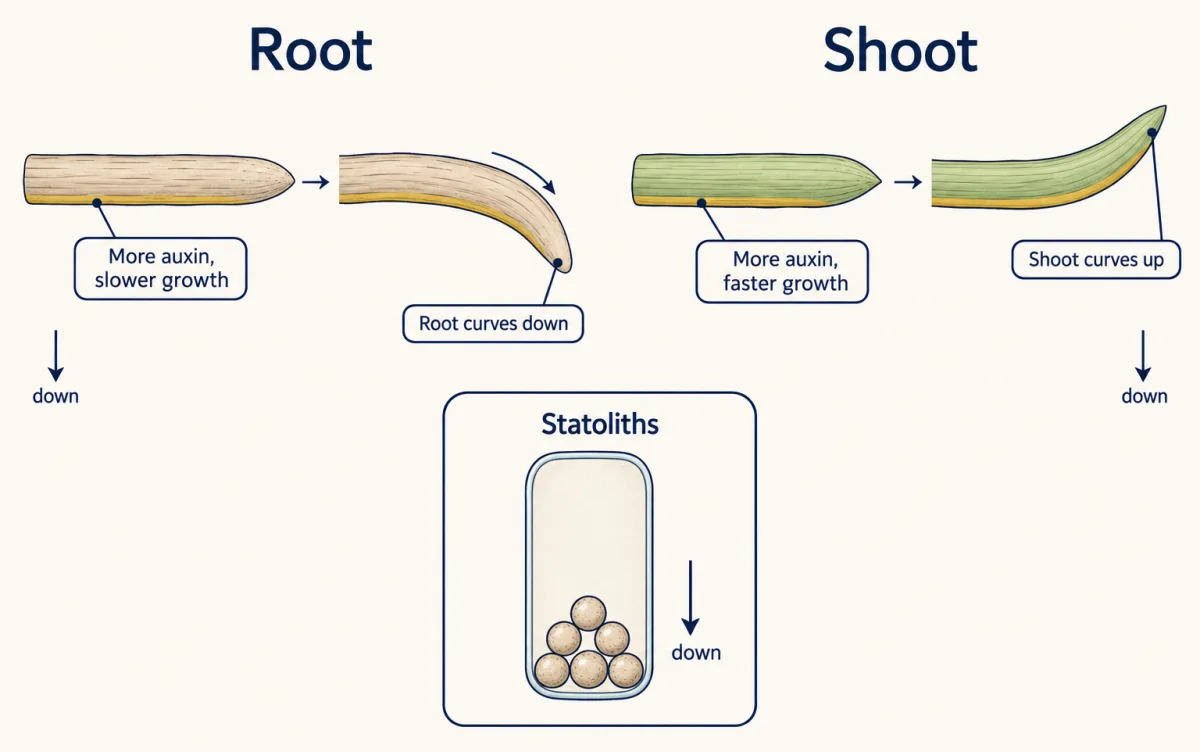
Gravitropism is a growth response to gravity. Lay a seedling on its side, and the shoot curves up while the root curves down.
Sensing starts with weight. In the central cells of the root cap, the columella, and in a starch sheath in shoots, plastids packed with dense starch act as statoliths: when Caspar and Pickard (1989) inverted wild-type Arabidopsis seedlings, these plastids sank toward the new lower side. Vertebrates use the same physics: in the inner ear, dense crystals shift with gravity and bend sensory hair cells (sensory coding). Statoliths are not the only sensor: starchless Arabidopsis mutants grown in light kept substantial root gravitropism.
In Arabidopsis root columella cells, PIN3 relocated quickly to the new lower face after the root was turned (Friml and colleagues, 2002), redirecting auxin toward the lower side.
The two organs respond in opposite ways to the same lower-side auxin. In the root, auxin inhibits elongation of epidermal cells on the lower side, the upper side grows faster, and the root curves down. In the shoot, extra auxin speeds elongation on the lower side, and the shoot curves up. The plant is not reaching for anything: each flank’s growth rate follows its auxin level, and the curve is the difference.
Light as information: phytochrome, night length and a travelling signal
Phytochrome is a pigment protein that switches between two forms. The Pr form absorbs red light and converts to Pfr; Pfr absorbs far-red light and converts back to Pr. In an assay of Arabidopsis phytochrome B, 660 nm light drove Pr to Pfr and 740 nm the reverse. In the simple model, Pfr is the active form. Pfr can also revert to Pr slowly in darkness. The lettuce-seed experiment that revealed this switch is the design problem.
Photoperiodism is a response to the relative lengths of day and night. A short-day plant flowers when nights are longer than a critical length; a long-day plant flowers when nights are shorter. Karl Hamner and James Bonner (1938) varied light and dark periods separately in cocklebur, Xanthium, a short-day plant. They reported that flowering depended mainly on the length of the dark period, and that the leaves perceived the inductive treatment. Flowers form at the shoot apex, so a signal must travel there from the leaf.
In Arabidopsis, a long-day plant, part of the signal is known. The protein CONSTANS is stabilized by light in the evening and degraded in the morning or in darkness, so it builds up only when days are long enough to be lit in the evening. CONSTANS then promotes transcription of the gene FT in the leaf phloem. Corbesier and colleagues (2007) showed that FT protein made in phloem moves to the shoot apex, including across grafts. The daily clock behind this is in sleep and rhythms, and flowering itself in plant reproduction. Do not assume the CONSTANS mechanism applies to cocklebur: it was worked out in Arabidopsis.
Signals of attack
Unlike vertebrates, plants have no circulating immune cells; each cell defends itself, and hormones spread the alarm. In Arabidopsis, a triple mutant with almost no jasmonate was attacked by larvae of the fungus gnat Bradysia impatiens, and applied methyl jasmonate substantially protected it. In tomato, caterpillars or moths that merely brushed and broke leaf hairs switched on jasmonate-regulated defence genes before any chewing.
Salicylic acid works in systemic acquired resistance, in which an infection in one part of a plant leaves uninfected parts more resistant to later attack. In tobacco infected with tobacco mosaic virus, salicylic acid was necessary for this response in the transgenic plants tested.
“Jasmonate for insects, salicylic acid for pathogens” is a tendency from tested systems, not a rule. The receptors that first detect a pathogen are shared logic with animals, and innate immunity covers them: surface receptors start pattern-triggered immunity, mostly intracellular receptors start effector-triggered immunity, and in Arabidopsis the two arms depend on each other.
Design problem
Lettuce seeds soaked in the dark get brief flashes of light, return to the dark, and germination is scored. Illustrative results, one seed batch, equal flash doses: dark only, 10%; red, 90%; red then far-red, 15%; red, far-red, red, 88%; red, far-red, red, far-red, 18%. What do they tell you, and what do they not?
One way to do it
Look at the last flash. Sequences ending in red give 88 to 90% germination; sequences ending in far-red give 15 to 18%, close to the dark control. Total light does not decide it: four flashes ending in far-red germinate less than one red flash.
The simplest explanation is one pigment that switches reversibly between two forms. Red light converts it to a form that promotes germination, and far-red light converts it back to the inactive form. This is the logic of Borthwick, Hendricks and colleagues’ 1952 Grand Rapids lettuce experiments.
The dark seeds, equal doses and a single batch make the reading safe: differences come from the order of flashes, not the seeds.
The data do not identify the pigment chemically, and do not show that other seeds respond the same way; many need no light to germinate.
How we measure it
Tip covering and barrier experiments
Cover a seedling tip with an opaque cap or a transparent tube, or insert an impermeable sheet such as mica into a cut on one side, then light the seedling from one side. Comparing the treatments shows where light is sensed and which route the signal takes, provided a control shows the covering or cut alone does not stop growth.
Oat coleoptile curvature bioassay
Let excised tips release their growth substance into agar, then place the block on one side of a decapitated coleoptile in the dark and measure the angle of curvature. Within a calibrated range, more curvature means more auxin activity in the block.
Sequential red and far-red light treatments
Give imbibed seeds or plants brief flashes of red or far-red light in different orders, with dark controls, and score germination or flowering. A response set by the last flash points to a pigment that switches reversibly between two forms.
Grafting with tagged proteins
Join the shoot of one plant to another, or make a protein carrying a visible tag only in certain cells, and look for the tag elsewhere. Finding a phloem-made FT protein at the shoot apex shows that the protein itself can travel.
Finish line
Test yourself
8 questions
Practice and MCAT-style, with explained answers.
Next · Lesson 26
Flowers, Seeds and Fruit
Every pollen grain delivers two sperm, and in a flowering plant both of them fertilize something. Why two?
Continue →