Organismal Biology · Unit 6: How plants work
Soil, Nutrients and Partners
A plant makes every organic molecule it contains from carbon dioxide, water and a short list of mineral elements, so what must it get from the soil, and how does it get it? This lesson lists the 17 elements conventionally essential to vascular plants, reads a sick leaf by where the symptoms appear first, follows water and ions into the root past the endodermis, and compares plants that take nitrogen and phosphorus from bacteria, fungi, insects or other plants. Afterwards you can design a test of essentiality, diagnose a deficiency from leaf age, and calculate how much surface root hairs and fungal hyphae add to a root.
Watch first Peas Borrow Nitrogen From Bacteria · 2:47
Peas grown in sterilised sand, given a little soil extract and watered with a solution that held no nitrogen, ended up with many times more nitrogen than their seeds contained. Oats in the next pot starved. Nitrogen gas makes up most of the air around both plants, so why could one use it and the other not? Answering that takes you through what a plant takes from the soil, how a root lets it in, and the partners some plants rely on.
What a plant must get from the soil
Start with a contrast to animals. You must eat certain amino acids and vitamins because your cells cannot make them, as digestive systems explains. A green plant builds every organic molecule it contains, every amino acid, lipid and nucleotide, from carbon dioxide, water and a short list of mineral elements. Photosynthesis fixes the carbon in the leaf; the chemistry of that belongs to the Calvin cycle. What the plant cannot make is an element. It has to take each one in.
An element is essential if, without it, a plant cannot complete its life cycle from seed to seed. Daniel Arnon and Perry Stout added two more conditions in 1939: no other element can stand in for it, and it acts directly in the plant rather than by changing the soil or its microbes.
The conventional list for vascular plants has 17 essential elements:
- From air and water: carbon, hydrogen and oxygen.
- Macronutrients (required in larger amounts): nitrogen, phosphorus, potassium, calcium, magnesium and sulfur.
- Micronutrients (required in trace amounts): chlorine, boron, iron, manganese, copper, zinc, nickel and molybdenum.
Some tables list 20. The extra elements are beneficial: they improve growth in some species but are not universal requirements. Sodium helps some plants with C4 or CAM photosynthesis, silicon strengthens grasses such as rice, and cobalt is used by the nitrogen-fixing bacteria in legume nodules.
The list was built in water culture. Dennis Hoagland and Arnon published a standard nutrient solution in 1938, and leaving one element out of it, then putting it back, is still the basic test.
Reading a sick leaf
A deficiency shows on the leaves, and where it shows first is a clue. The key is mobility: whether the plant can move an element out of old tissue and through the phloem to growing tissue.
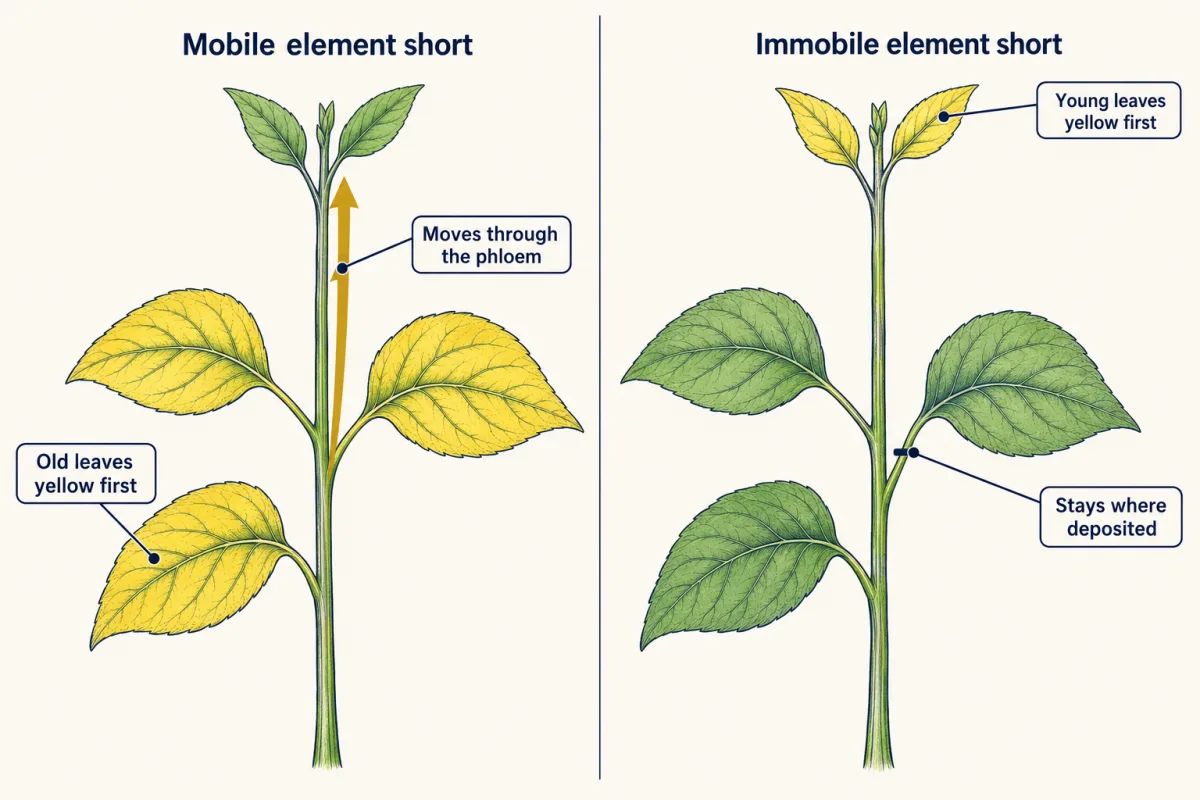
- Mobile elements (nitrogen, phosphorus, potassium, magnesium) are withdrawn from old leaves when supply runs short. Symptoms appear first in old, lower leaves.
- Immobile elements (iron and calcium, and boron in most species) stay where they were deposited. New leaves get only what arrives from the roots, so symptoms appear first in young leaves and growing tips.
Here chlorosis means yellowing from lost chlorophyll, and necrosis means patches of dead tissue.
A study of Japanese mint (Mentha arvensis), grown in greenhouse hydroponics with one nutrient left out of Hoagland’s solution at a time, shows the pattern. Without nitrogen, the whole blade of old leaves yellowed first, with symptoms first seen 15 days after transplanting. Without iron, young leaves yellowed. Without potassium, old leaves developed yellow spots. Without phosphorus, blades turned dark green with purple margins. In sweetgum, magnesium deficiency can yellow the tissue between the veins while the veins stay green.
Treat these as examples, not a key for every species. Different deficiencies can look alike, and drought, disease or cold can mimic them. A symptom is a hypothesis. Tissue analysis, measuring the elements in the leaf, tests it, and add-back, supplying the suspected element and watching new growth recover, confirms it.
Into the root: hairs, two routes and a gatekeeper
Most uptake happens near the root tip, where root hairs, tubular outgrowths of single epidermal cells, push into the spaces between soil particles and enlarge the absorbing surface.
Worked problem: how much surface do hairs and hyphae add? These are illustrative numbers, not measurements from one species. Treat every structure as a cylinder and ignore the ends.
side area of a cylinder = pi x d x L surface per volume of a cylinder = 4 / d
- The root. A 10 mm segment, 0.5 mm in diameter: pi x 0.5 mm x 10 mm = 15.7 mm2.
- The hairs. Suppose 1,000 hairs on that segment, each 0.5 mm long and 0.010 mm wide. One hair: pi x 0.010 mm x 0.5 mm = 0.0157 mm2. All of them: 1,000 x 0.0157 = 15.7 mm2. The hairs double the surface, to 31.4 mm2.
- The fungus. Suppose 1 m (1,000 mm) of mycorrhizal hyphae, each 0.004 mm wide, attached to the segment: pi x 0.004 mm x 1,000 mm = 12.6 mm2. The total is now 15.7 + 15.7 + 12.6 = 44.0 mm2.
- Surface per material. With 4 / d, the root gives 4 / 0.5 = 8 per mm, a hair 4 / 0.010 = 400 per mm and a hypha 4 / 0.004 = 1,000 per mm. Check by volume: the hyphae occupy pi x (0.002 mm)2 x 1,000 mm = 0.013 mm3, against 2.0 mm3 for the root segment. They add more than three quarters of the root’s own surface for under one per cent of its volume.
Surface matters most for ions that move slowly through soil. Phosphate diffuses so slowly that a root soon empties the soil right around it, and thin hyphae reach past that emptied zone. Hairs help with water too, but not equally everywhere: in barley, root hairs aided water extraction by rapidly transpiring plants in drying soil, while a hairless maize mutant took up water no differently in sand or loam. (Moving water and sugar in plants covers water potential and the pull of transpiration.)
In this sketch: illustrative numbers, not a measured species; every structure is a cylinder; ends ignored; not to scale; drawn lines are a sample, not a count.
Side area of a cylinder = π × d × L, and surface per volume of a cylinder = 4 / d, so the thinner the cylinder, the more surface per unit of material.
Inside the root, water and dissolved ions cross the cortex by two routes. The apoplast is the continuous network of cell walls and spaces outside the membranes. The symplast is the cytoplasm of cells joined by plasmodesmata, channels through the walls. Both routes reach the endodermis, the innermost cortical layer around the central cylinder. In the walls between endodermal cells runs the Casparian strip, a band that blocks the wall route. In young Arabidopsis roots that band is lignin, not suberin as older textbooks say; suberin is laid down later. Past the strip, anything heading for the xylem has to cross a living membrane, so the endodermis acts as a gatekeeper on what enters.
Taking up many nutrient ions takes energy, because they often move against their gradients. A proton pump, an ATP-driven H+-ATPase of the P type in the plasma membrane, moves protons out of root cells. Transporters then let a proton flow back in with nitrate or another ion, cotransport. In Arabidopsis the NRT1.1 nitrate transporter works this way. How such transporters work is in membrane transport.
Borrowing nitrogen and phosphorus: nodules and mycorrhizae
Back to the peas. At the Bernburg experiment station, Hermann Hellriegel and Hermann Wilfarth grew legumes, including peas, and cereals, including oats, in sterilised sand with a nitrogen-free nutrient solution, and published the work in 1888. If every plant relied on nitrogen compounds in soil, none should end with more nitrogen than its seed held. The cereals grew only as far as the nitrate they were given allowed. Peas given a little extract of field soil formed nodules, swellings on the roots, and gained much nitrogen from the air. Without the extract, or with extract that had been heated, they formed no nodules and did not. A living agent from soil, tied to the nodules, was required. The experiment did not identify the agent; in the same year Martinus Beijerinck reported isolating bacteria from nodules.
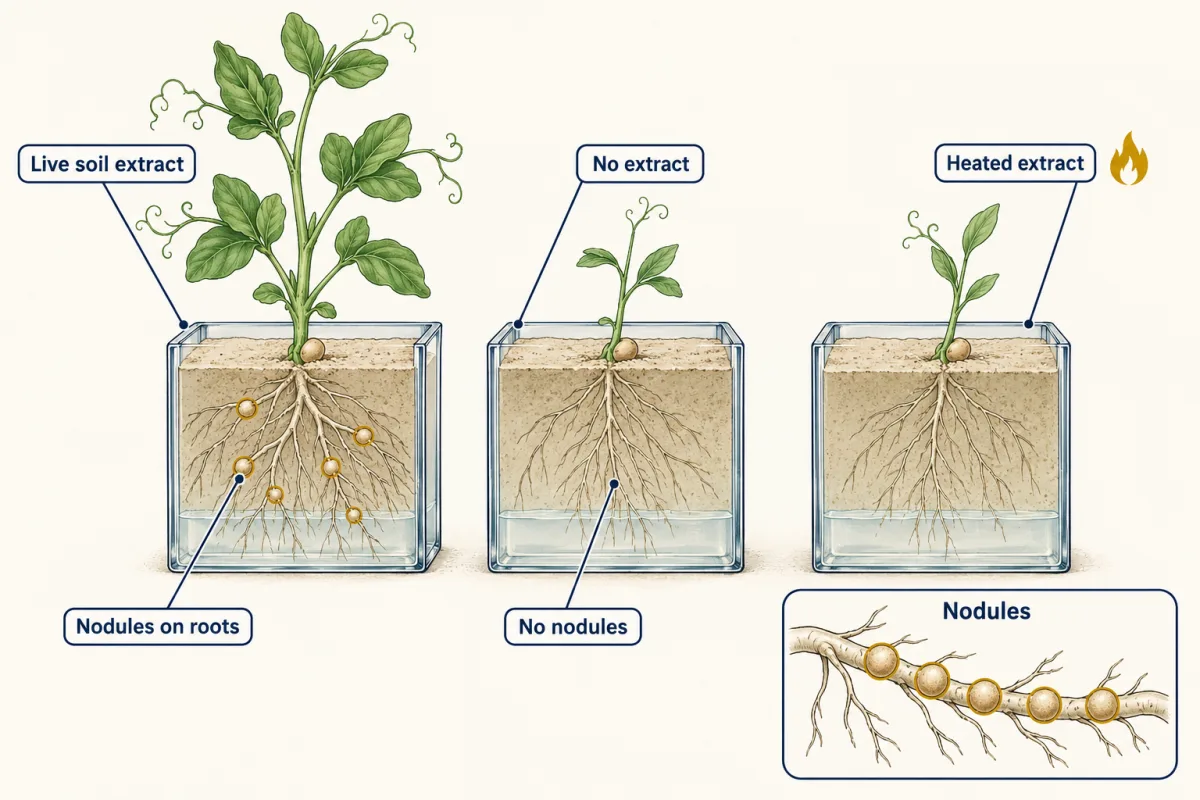
Those bacteria are rhizobia. They enter the root, and inside nodule cells they become bacteroids whose enzyme, nitrogenase, reduces nitrogen gas to ammonia. The root makes no nitrogenase. In return the plant supplies carbon: sucrose from the leaves is converted to malate, which fuels the bacteroids. Nitrogenase is damaged by oxygen, yet the bacteroids respire. A plant protein, leghemoglobin, binds oxygen and buffers it at a low, steady level. It does not exclude oxygen. In Lotus japonicus, Ott and colleagues (2005) silenced leghemoglobin: free oxygen in nodules rose, fixation stopped, and the plants grew normally only when given mineral nitrogen. Oats and barley have no nodules and depend on nitrate and ammonium in the soil. The ecosystem side of fixation is in nutrient cycling.
Phosphorus is borrowed from fungi. A mycorrhiza is an association of a root with a fungus (fungal hyphae appear in microbes, protists and fungi).
- Arbuscular mycorrhizae form in most land plants. Hyphae enter cortex cells and branch into arbuscules, tree-like structures where nutrients are released. In Lotus japonicus with the fungus Rhizophagus irregularis, the fungus delivers minerals taken from soil, especially phosphate. Keymer and colleagues (2017) showed with isotope labelling and plant mutants that the plant pays in lipids as well as sugars.
- Ectomycorrhizae form on trees such as pines and oaks. The fungus wraps the root tip in a sheath and grows between cortex cells without entering them.
Partners differ in quality, and hosts can respond to that, as mutualism, parasitism and coevolution explains.
Plants that eat animals and plants that tap plants
The purple pitcher plant, Sarracenia purpurea, grows in nitrogen-poor bogs. It photosynthesizes like any green plant, and its flat leaves, phyllodia, photosynthesize more efficiently than its pitchers. Insects drown in rainwater held in the pitchers, where bacteria, protists and larvae break them down, releasing mineral nitrogen and also competing with the plant for it. Karagatzides, Butler and Ellison (2009) added labelled amino acids to pitchers in Ontario and Massachusetts and found data consistent with direct amino-acid uptake by the plant, clearest for phenylalanine.
Dodder (Cuscuta) takes a different route. This twining stem parasite forms haustoria, organs that grow into the host stem and connect to its xylem and phloem, drawing water, nutrients and sugars.
A pea borrows from bacteria, a pine from fungi, a pitcher plant from insects and a food web, and dodder from another plant. In those pots, oats had only the nitrate their solution held.
Design problem
Brown, Welch and Cary (Plant Physiology, 1987) asked whether nickel is essential for barley (Hordeum vulgare, cultivar Onda). Nickel is needed in such small amounts that contamination from salts, water and the seed itself can hide a requirement. Design the test.
One way to do it
Grow barley in solution culture made with purified salts and clean water, so the solution is depleted of nickel. Give one group no added nickel and a second group the same solution plus nickel, and keep a third group of deficient plants for later add-back. Run the experiment for the whole life cycle and into the next generation, because a seed carries nickel from its mother, and a first-generation plant may live on that store. Measure grain nickel and test whether the grain germinates. In the published experiment, adding nickel completely relieved the deficiency symptoms in the mother plants, and grain with less than 30 ng of nickel per gram of dry weight was not viable. Failure without nickel and rescue with it meet the Arnon and Stout criterion of a life cycle that cannot be completed without the element. The limits: this was one cereal in one preparation, so it does not give a threshold for all plants or any fertiliser rate.
How plants sense and respond to what they find, through hormones, comes next in plant signals.
How we measure it
Solution culture with omission and add-back
Grow plants in a complete nutrient solution made from purified salts, and in matching solutions each lacking one element, then add the element back to some deficient plants. A symptom that appears on omission and disappears on add-back ties the symptom to that element in that species.
Tissue elemental analysis
Dry and dissolve leaf or grain tissue and measure its elements, today often by inductively coupled plasma mass spectrometry (ICP-MS). It tests a diagnosis made from symptoms, since different deficiencies can look alike.
Stable-isotope pulse-chase
Supply a compound labelled with a heavy isotope, such as nitrogen-15 in amino acids, and measure where the label turns up over the following hours or days. It shows which route a nutrient took into a plant or between partners.
Tracer dye exclusion at the endodermis
Bathe roots in a dye such as propidium iodide that travels in cell walls but does not cross intact membranes, and look under the microscope for whether it reaches the central cylinder. An intact Casparian strip stops it at the endodermis.
Finish line
Test yourself
8 questions
Practice and MCAT-style, with explained answers.
Next · Lesson 25
Plant Hormones and Responses
Light an oat seedling from one side and it bends toward the lamp. The tip senses the light, yet the bend forms lower down. What told it?
Continue →