Organismal Biology · Unit 6: How plants work
Flowers, Seeds and Fruit
How does a plant that cannot move get its sperm to an egg, and its offspring away from itself? This lesson names the parts of a flower, follows pollen from anther to ovule, explains why a flowering plant fertilizes twice, and traces the ovule to a seed and the ovary to a fruit. Afterwards you can count the chromosomes in every part of a maize kernel, predict kernel colours from a cross, and judge what evidence a claim of flower-pollinator coevolution needs.
Watch first One Tube, Two Sperm, Two Fusions · 2:29
Shake a ripe maize tassel and a yellow haze drifts off. Each grain is not a sperm but a tiny plant of three cells, and if it lands on a silk it grows a tube the length of the silk and delivers two sperm, both of which fertilize something.
Why two? And how does a plant rooted in one spot get sperm to an egg on another plant, and its offspring away from itself? This lesson follows a flowering plant from flower to seed to fruit.
The parts of a flower: four rings of organs
A flower is a short shoot that bears the reproductive organs of a flowering plant (an angiosperm). Typically the organs sit in four rings, or whorls, on the swollen tip of the flower stalk, the receptacle. From the outside in:
- Sepals, together called the calyx, are often green and enclose the bud.
- Petals, together the corolla, are often coloured.
- Stamens are the male organs. Each is a stalk, the filament, holding an anther, where pollen forms.
- Carpels are the female organs. A carpel has a sticky tip, the stigma, a neck, the style, and a swollen base, the ovary, which holds one or more ovules.
Not every flower has all four whorls. Maize has male flowers in the tassel and female flowers on the ear, and each silk is a long style.
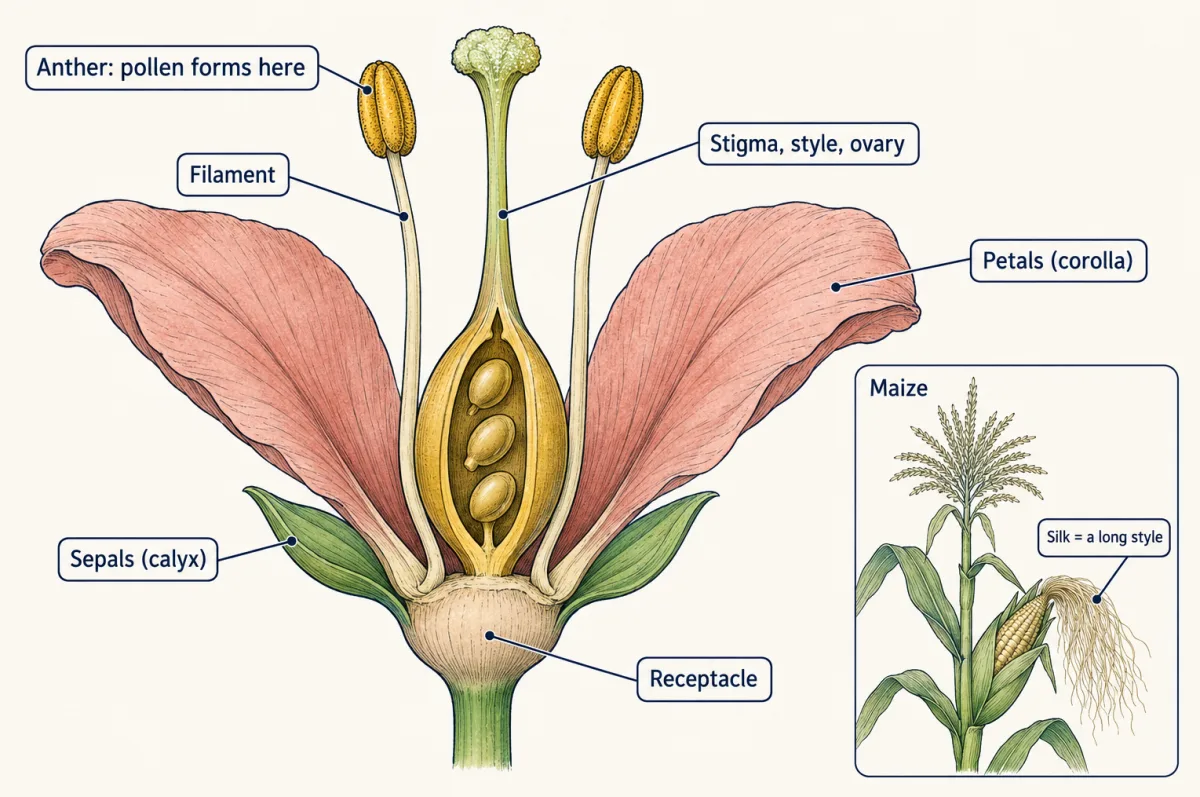
Pollen forms in the anther. A diploid microspore mother cell divides by meiosis (see chromosomes and meiosis) into four haploid microspores. Each microspore divides by mitosis into a large tube cell and a small generative cell inside it, and the generative cell divides again into two sperm. In Arabidopsis and maize this happens before the pollen is shed, so the grain has three cells; in lilies the grain is shed with two cells and the sperm form inside the growing tube.
A pollen grain is therefore a male gametophyte, reduced to two or three cells. Recall alternation of generations from plants on land: a life cycle in which a diploid spore-making plant (the sporophyte) alternates with a haploid gamete-making one (the gametophyte).
The female gametophyte is the embryo sac, inside the ovule: in Arabidopsis, eight nuclei form seven cells, including two synergids beside the egg and a large central cell whose two polar nuclei fuse. Around it lie one or two layers of maternal tissue, the integuments, which leave a small opening, the micropyle.
Pollen meets pistil: one tube, two fertilizations
Pollination is the transfer of pollen from an anther to a stigma. Fertilization is the fusion of a sperm with a female cell inside the ovule. They are separate events: a flower can be pollinated and never fertilized.
On a compatible stigma the grain takes up water, and the tube cell grows a pollen tube down through the style into the ovary. The sperm, which have no flagella, ride inside it. Near the ovule the tube follows chemical signals released by the synergids, enters the ovule, usually through the micropyle, and bursts into one synergid, releasing its two sperm.
In double fertilization, one sperm fuses with the egg, giving a diploid zygote, which grows into the embryo. The other fuses with the central cell, giving the first cell of the endosperm, a tissue that stores food for the embryo. In Arabidopsis, maize and most flowering plants the central cell carries two haploid polar nuclei, so the endosperm is triploid (3n). Not in every species: in water lilies, for example, the central cell has a single polar nucleus and the endosperm is diploid.
Compare animals (animal reproduction): in most, one sperm fuses with one egg, and the sperm usually swims to it. A flowering plant delivers non-swimming sperm through a tube, and fertilizes twice, as Sergei Navashin (1898) and Léon Guignard (1899) saw in lily ovules.
Worked problem: counting chromosomes and kernel colours in maize. Maize (Zea mays) has 2n = 20. Assume one gene for endosperm colour, with yellow (Y) fully dominant over white (y); in real maize the yellow deepens with each extra Y copy.
- Chromosome counts. Egg: 10. Each sperm: 10. Central cell with two polar nuclei: 10 + 10 = 20. Zygote and embryo: 10 + 10 = 20. Endosperm: 20 + 10 = 30. Seed coat and fruit wall are the mother plant’s own tissue: 20.
- A cross with a surprise. A white-kernelled yy plant is pollinated with pollen from a YY plant. The egg is y, the polar nuclei are y and y, and the sperm carry Y. The embryo is Yy and the endosperm is yyY, so the kernels are yellow, on a plant whose selfed kernels would be white. Kernel colour comes from the endosperm, a product of fertilization, so the pollen parent’s genes show in this generation’s seed. This is called xenia.
- Selfing a heterozygote. A Yy plant self-pollinates and an ear sets 400 kernels. In maize the egg and both polar nuclei descend by mitosis from one megaspore, so the central cell is YY when the egg is Y and yy when it is y, each with probability 1/2. The sperm carries Y or y, each 1/2, independently (probability and crosses), so the endosperm is YYY, YYy, yyY or yyy, each 1/2 x 1/2 = 1/4. Only yyy is white. Expected, assuming random fertilization and equal kernel survival: 3/4 x 400 = 300 yellow and 1/4 x 400 = 100 white (check: 300 + 100 = 400).
Letters in teal are copies from the seed parent (maternal); letters in orange are copies from the pollen parent (paternal). In this sketch, both polar nuclei and the egg descend from one megaspore (as in maize), and both sperm of one grain carry the same allele. Showing the kernel you select on the ear below.
yellow kernel white kernel selected kernel (click it, or use the arrow keys). Kernels drawn as a grid of dots.
| Endosperm (central cell + sperm) | Kernel colour | Expected of 400 | Simulated |
|---|
In this sketch: one gene, with yellow (Y) fully dominant over white (y), though in real maize the yellow deepens with each extra Y copy; every ovule is fertilized; kernels are independent; counts on the ear are random draws made by this sketch, not data; expected counts assume random fertilization and equal kernel survival. Zea mays, 2n = 20.
Rule to keep: endosperm = 2 maternal sets + 1 paternal set; embryo = 1 maternal set + 1 paternal set. Seed coat and fruit wall are the mother plant’s own tissue and never take the pollen’s genotype.
endosperm = 2 maternal sets + 1 paternal set; embryo = 1 maternal set + 1 paternal set
Flowers and their animals: wind, insects and coevolution
Grasses such as maize, and oaks, are pollinated by wind. Their flowers have small petals or none and no nectar, with exposed stigmas, and they shed huge amounts of light, dry pollen, almost all of which lands nowhere useful. Field mustard, Brassica rapa, is pollinated by bees and hoverflies. Its petals, scent and nectar attract visitors, and its sticky pollen travels on them to the next flower.
Self-pollination moves pollen to a stigma of the same flower or the same plant; outcrossing moves it to another plant. Selfing is still sexual reproduction: it uses meiosis and fertilization, and a heterozygous plant’s selfed offspring vary. Many species have self-incompatibility, a recognition system in which the stigma or style rejects pollen carrying the plant’s own incompatibility alleles; wild B. rapa is an example.
Coevolution is reciprocal evolutionary change between interacting lineages: each changes in response to the other (see mutualism, parasitism and coevolution). Darwin’s Madagascar orchid, Angraecum sesquipedale, holds its nectar at the bottom of a spur nearly 30 cm long. In 1862 Darwin predicted a moth with a tongue long enough to reach it, and in 1903 Rothschild and Jordan described the hawkmoth Xanthopan morganii praedicta. A match like this is a hypothesis. Coevolution needs evidence on both sides: that moths selected on spur length, and that flowers selected on tongue length. If the tongue lengthened for other reasons and the orchid tracked it, that is one-sided adaptation. The design problem below tests the plant side in Brassica rapa.
From ovule to seed, ovary to fruit
After fertilization the ovule becomes the seed, and in most flowering plants the ovary becomes the fruit, which encloses the seeds. A seed has three parts of three origins. The embryo, a new diploid plant with a root tip, a shoot tip and one or two seed leaves (cotyledons), comes from the zygote. The food store comes from the endosperm. The seed coat comes from the integuments, so it is the mother’s tissue. In maize and wheat grains the endosperm persists and holds the starch; in beans, peas and shepherd’s purse (Capsella) the cotyledons absorb the endosperm as the seed develops and store the food themselves.
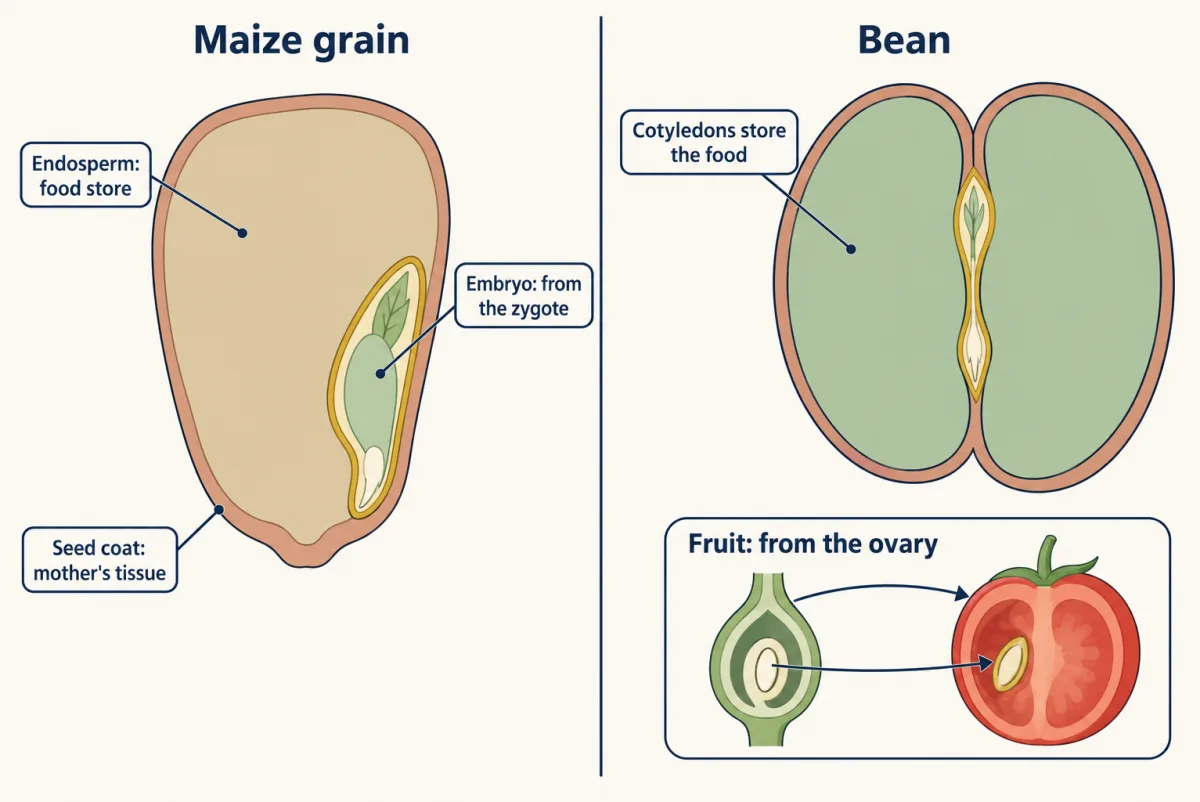
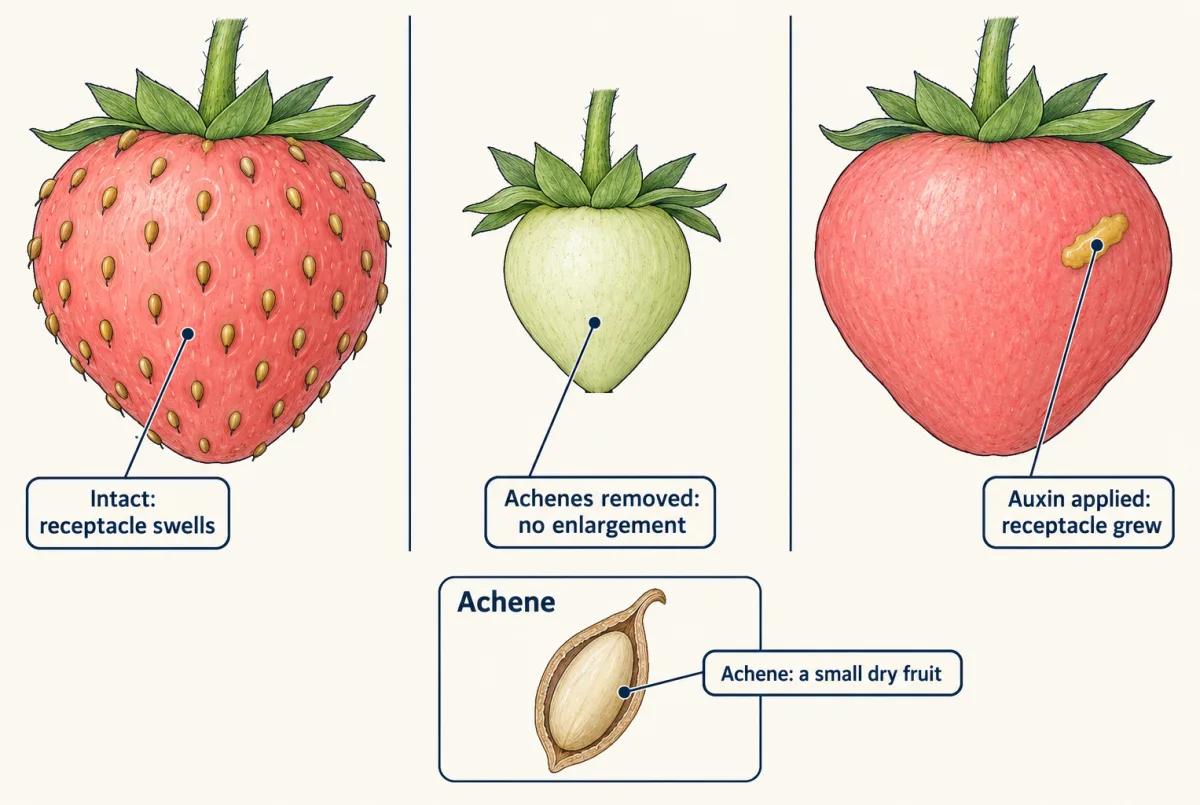
A tomato’s flesh is ripened ovary wall. A strawberry is an accessory fruit, one whose flesh comes from tissue other than the ovary: the red part is the swollen receptacle, and the specks on its surface are achenes, each a small dry fruit holding one seed.
Why does a strawberry receptacle swell only after pollination? Jean Paul Nitsch tested this in 1950 on young pollinated receptacles. If the receptacle grew on its own once the flower was pollinated, removing the achenes would make no difference. Instead, receptacles stripped of achenes did not enlarge. And stripped receptacles treated with an auxin, a plant hormone (see plant hormones and responses), grew. That rules in a signal from the achenes that auxin can mimic, and rules out receptacle growth independent of them. It does not show that the signal is auxin alone, or how it moves. In Fragaria vesca, Tian and colleagues (2022) found that a gibberellin-synthesis blocker reduced the enlargement caused by applied auxin, and auxin transport from achene to receptacle remains a proposed model.
Waiting and travelling: dormancy, dispersal and clones
Seed dormancy is the failure of an intact, viable seed to complete germination under favourable conditions. In the framework used in Arabidopsis seed studies, the hormone abscisic acid (ABA) is required to induce dormancy as the seed matures, and gibberellins promote germination, which begins when the seed takes up water and ends when the embryonic root pushes out through the seed’s coverings.
Dandelion fruits carry a parachute of fine hairs and drift on the wind. Coconut fruits float and travel by sea. Jays and squirrels bury acorns and fail to recover some, which germinate away from the parent oak.
Many plants also reproduce asexually. Strawberry stolons, or runners, are horizontal stems that root at their nodes into new plants. Potato tubers are swollen underground stems whose buds, the eyes, sprout. Apomixis is seed formation without meiosis and fertilization, giving an embryo that is a clone of its mother. Liu and colleagues (Plant Communications, online 2022) followed engineered apomictic lines of the hybrid rice Chunyou 84 for four generations: 1.9 to 3.2% of tested offspring were clones, and in one field season seed set was 5.7 to 7%, against 75.9% for the unedited hybrid.
Design problem
Gervasi and Schiestl (2017) let fast-cycling Brassica rapa be pollinated only by bumblebees, only by hoverflies, or by hand, with three replicate populations of 36 plants per treatment. After nine generations of selection and a round of crosses between replicates within each treatment, they compared the plants of generation 11. Bumblebee-pollinated plants became taller, and bumblebees preferred them in a choice test. Hoverfly-pollinated plants self-pollinated more. Is this coevolution? What does each part of the design rule out, and what more would you need?
One way to do it
The hand-pollinated lines shared the greenhouse, so traits that changed only in the insect lines are not explained by greenhouse conditions. Three replicates test repeatability: drift, random change in small populations, would push replicates in different directions, while selection by one pollinator should push them the same way.
So pollinators can drive plant evolution quickly. One hypothesis for the hoverfly result: where a pollinator delivers little outcross pollen, plants that selfed may leave more offspring.
It is not evidence of coevolution. Only the plants were followed, so one side of a reciprocal change was tested; you would also need insects evolving alongside, with traits that changed in response to the plants. And one pollinator in a greenhouse is not a field community, so the result shows what pollinators can do, not what they do in a meadow.
How we measure it
Fixed, sectioned and stained ovules under the light microscope
Collect ovules at timed stages after pollination, fix and slice them thin, and stain the nuclei. A series of stages lets you infer the order of events, such as which male nucleus joins which female cell, though each section is a snapshot rather than a film.
Organ removal and hormone replacement
Remove a structure suspected of sending a signal (here the achenes of a strawberry), see what fails, then apply a candidate hormone in its place. If the hormone restores the response, the structure supplies a signal the hormone can mimic; it does not prove the hormone is the natural signal.
Replicated experimental evolution
Found several populations, give each a different selective regime (here, which animal pollinates), and add a control regime such as hand pollination. Differences that arise in every replicate of a treatment, and not in the controls, point to selection rather than drift or greenhouse conditions.
Laser ablation with live imaging
Destroy one chosen cell with a focused laser pulse and film what the remaining cells do. In dissected Arabidopsis ovules this tests whether fertilization of the central cell depends on a working egg.
Finish line
Test yourself
8 questions
Practice and MCAT-style, with explained answers.
That's the last lesson
Back to all lessons
Pick another topic, or revisit one you want to firm up.
All lessons →