Organismal Biology · Unit 1: Organisms and their diversity
What an Organism Has to Do
Every multicellular organism, from a barley plant to a human, faces the same short list of problems: getting energy and materials, exchanging and moving them (wastes included), keeping its inside relatively stable, resisting damage and invasion, and leaving descendants. This lesson sets out that list as the frame for the course, uses the barley leaf and the human lung to show that every exchange surface carries a cost, and separates how questions from why questions. Afterwards you can calculate a water-use efficiency, say why structure fits function without calling it design, and sort an explanation into proximate or ultimate.
Watch first Every Exchange Surface Has a Cost · 2:55
A barley leaf cannot take in carbon dioxide without letting water out. The gas enters through tiny pores, and water vapour leaves through the same pores. Your lungs face a version of the same bargain. This first lesson asks what every multicellular organism has to manage, and why its solutions always carry a cost.
Five problems, one checklist for the course
A multicellular organism is a body built of many cells that depend on one another. Barley, honeybee or human, it faces the same few recurring problems, and this course uses five as a checklist. The list is a teaching frame, not an official definition; other books divide the ground differently.
- Energy and materials. All organisms use an energy source to run their chemistry. Animals get theirs from food they ingest or absorb. Plants capture light energy and fix carbon from the air in their leaves (the chemistry is in the light reactions), but the roots of seed plants also absorb water and minerals from the soil. The oxygen a plant gives off is a by-product of splitting water during photosynthesis.
- Exchange and transport, including wastes. Materials must cross a surface and reach every cell, and wastes must leave. In a small organism, diffusion, the net movement of molecules from higher to lower concentration, can do much of this. In a large one it cannot reach far enough, and transport systems carry the load: blood vessels in animals, and in plants the xylem (tissue that carries water and minerals up from the roots) and the phloem (tissue that carries sugars from where they are made to where they are used). Size, scale and surface shows why size forces this, and gas exchange and moving water and sugar in plants show the solutions.
- Control and relative internal stability. Homeostasis is the maintenance of a relatively stable internal environment. Adult humans hold their core temperature near 37 degrees C; a plant closes its stomata when its leaves run short of water. Tissues, organs and homeostasis builds this out.
- Defense. Bodies are damaged and invaded. In the small plant Arabidopsis, closing the stomata can be part of the defense against bacteria that enter through those pores. Animals have skin, mucus and immune cells, the subject of innate immunity.
- Reproduction, as continuation of a lineage. Reproduction passes DNA, and the genes it carries, to offspring. It is a problem for the lineage, not for every individual. In honeybees, workers rarely reproduce while a queen is present, and in many other eusocial species (animals that live in colonies with a division of reproductive labour) the workers reproduce little or not at all, yet their colonies go on producing queens and males.
One leaf, one lung: the gas-for-water trade-off in two lineages
A surface that passes gas from air to living cells, as in a leaf or a human lung, has to be thin and wet, because the gas has to dissolve in a film of water before it can diffuse into cells. A wet surface exposed to air loses water by evaporation. Two lineages show the coupling.
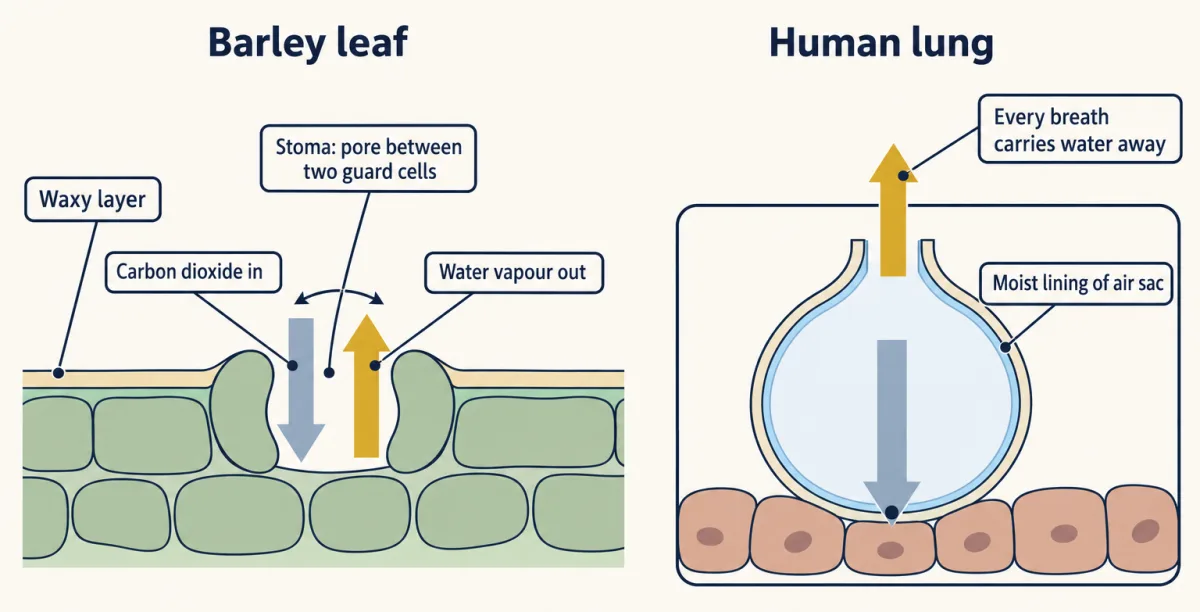
In barley (Hordeum vulgare), the leaf surface is covered by a waxy layer that water crosses poorly. Gas moves mainly through stomata (singular stoma), pores each flanked by two guard cells that open and close the gap. When stomata are open, carbon dioxide diffuses in toward the cells that fix it, and water vapour diffuses out. The loss of water vapour from leaves is called transpiration.
In an adult human, the exchange surface is the lining of the lung’s tiny air sacs. It is moist, and the air you breathe out is nearly saturated with water vapour, so every breath carries water away. The lung sits deep inside the chest, which shelters it, but it cannot close the way a stoma can. Neither solution escapes the cost.
The classic experiment. Hughes, Gray and colleagues asked what happens to barley with fewer stomata. They overexpressed a barley gene, HvEPF1 (overexpression means adding extra copies so the gene’s product is made in large amounts). This limited the entry of leaf cells into stomatal development and their progress through it. They compared two such lines with empty-vector controls, plants put through the same genetic procedure without the added gene. In the mature sixth leaf, the two lines kept about 24% and 12% of the control stomatal density. In a greenhouse, plants were grown at 60% or 25% on the authors’ calibrated soil-water scale.
You might expect less water lost and, with less carbon taken in, less grain. The first part held in well-watered plants: leaf gas exchange fell substantially (under water restriction, carbon assimilation and stomatal conductance (how freely gas passes through the stomata) did not differ significantly from controls). Water-use efficiency integrated over the life of the flag leaf (the uppermost leaf, just below the grain head), estimated from carbon isotopes in the leaf, rose in both lines under water restriction and in one line when well watered. The second part was not seen. With five plants per group, neither line showed a statistically significant drop in grain yield under either watering treatment. Two cautions. The instantaneous efficiency measure, assimilation divided by stomatal conductance, did not rise under water restriction. And five plants per group cannot prove the yields equal; it means no loss was detected. In a separate test where water was withheld, the engineered lines kept photosystem II, part of the light-capturing machinery, working about four days longer than controls.
Worked problem. These numbers are illustrative, not barley data. Leaf A assimilates 20 umol CO2 per m2 per s and transpires 5 mmol H2O per m2 per s. Leaf B has fewer stomata, under the same light and temperature, and assimilates 16 umol CO2 per m2 per s while transpiring 3 mmol H2O per m2 per s. Assume both rates stay constant.
water-use efficiency = carbon gained / water lost
- Efficiency. Leaf A: 20 / 5 = 4.0 umol CO2 per mmol H2O. Leaf B: 16 / 3 = 5.3 umol CO2 per mmol H2O.
- Compare. Leaf B gains 16 / 20 = 0.8 of A’s carbon, 20% less. It loses 3 / 5 = 0.6 of A’s water, 40% less. Its efficiency is 5.33 / 4.0 = 1.33 times A’s.
- Over a 10-hour day (36,000 s). Leaf A loses 5 mmol x 36,000 = 180,000 mmol = 180 mol H2O per m2, or 180 x 18 g per mol = 3,240 g, about 3.24 kg. Leaf B loses 3 x 36,000 = 108 mol, or 1,944 g, about 1.94 kg.
Neither leaf is better everywhere. When water is scarce, leaf B keeps more of it for each unit of carbon gained. When water is plentiful and carbon limits growth, leaf A gains more.
Bar scales: carbon gained 0 to 20 umol CO2 per m2 per s; water lost 0 to 5 mmol H2O per m2 per s; efficiency 0 to 20 umol CO2 per mmol H2O. Arrow widths follow the rates (schematic). The outline marks the bar the chosen condition is about, on the leaf that is ahead; none if tied.
In this sketch: illustrative numbers, not barley data; constant rates; same light and temperature for both leaves; 18 g of water per mol.
Water-use efficiency = carbon gained / water lost. In the lesson’s example neither leaf is better everywhere; which is better depends on whether water is scarce or carbon limits growth.
Why structure fits function, and why never perfectly
Structures usually fit what they do, and the explanation is historical. Natural selection acts on existing, inherited variation in a population. Over generations, it can increase the share of inherited traits associated with greater reproductive success. An adaptation is a heritable trait that helps survival and reproduction in its present environment. So “lineages with fewer stomata lost less water and left more descendants in dry places” is the right form for an evolutionary claim, and “the plant made fewer stomata to save water” is not. Such claims are tested in testing evolutionary explanations and selection in ecological context.
The fit is never perfect, for at least three reasons.
Trade-offs. A trade-off is a link between two traits such that improving one worsens the other. More stomata gain more carbon and lose more water. Lifetime trade-offs, such as reproducing early against growing larger, appear in life histories.
History. The human arm, the bat wing and the whale flipper share one pattern: an upper arm bone, two forearm bones, wrist bones and digits. They are homologous, inherited from a common ancestor and modified in each lineage, which you can read off a tree in reading phylogenetic trees. Selection on a whale’s ancestors could reshape those bones, but it began from them. Evolution does not move a population toward a preconceived ideal.
Chance and by-products. Not all evolutionary change is adaptive. Some traits spread by chance in small populations, and some are side effects of other features. Gould and Lewontin named the second kind after the spandrels of a Venetian cathedral: spaces left over between arches, later decorated, not built for the decoration.
So “perfectly adapted” is never the right phrase. No living organism is “more evolved” than another, either: a honeybee and a human have both had the same length of time since their common ancestor, and each lineage has its own solutions to the same five problems.
How questions and why questions
Ask “why does a barley leaf have the stomatal density it has?” and you can mean two different things. In 1961 Ernst Mayr distinguished proximate causes, which act within an organism’s lifetime, from ultimate causes, which lie in the lineage’s evolutionary history. In 1963 Niko Tinbergen split each kind in two, giving four questions:
| Kind | Question | Barley stomata |
|---|---|---|
| Proximate | Mechanism: how does it work now? | How guard cells open and close the pore |
| Proximate | Development: how does it form? | How genes such as HvEPF1 set how many stomata a leaf makes |
| Ultimate | Adaptive significance: what effect on survival and reproduction? | Whether density changes reproductive success in a given field environment |
| Ultimate | History: how did it change over the lineage? | How stomatal density changed across grasses on a tree |
The barley experiment answers a proximate, developmental question in engineered lines. It does not show how stomatal density evolved in wild barley, or field performance. A full account needs both kinds of answer, and neither replaces the other.
“Ultimate” does not mean purpose, although the word “why” can make a question sound as if it asks for an intention. An ultimate answer is a history of what happened to a lineage, such as which variants left more descendants.
Design problem
Guppies (Poecilia reticulata) in Trinidad streams live with many predators below some waterfalls and few above them. Reznick, Shaw, Rodd and Shaw (Science, 1997) reported on fish moved from high-predation sites into low-predation streams above waterfalls. At one site, El Cedro, males from the introduced population matured later than males from the source population within about four years. How would you show that this difference is inherited rather than a direct effect of food or water, and is that a proximate or an ultimate question?
One way to do it
Collect fish from the introduced population and, at the same time, from the source population, which serves as the control. Rear their descendants side by side in one laboratory environment, with the same food, temperature and density, for at least two generations; the study used second-generation laboratory fish. Two generations dilute effects passed on through the mother’s condition. If introduced-population males still mature later, the difference is likely inherited. In that assay the adjusted mean male maturation ages were 60.6 days for source fish and 72.7 days for introduced fish; measured female traits had not changed significantly at four years (later maturation had appeared in females by 7.5 years).
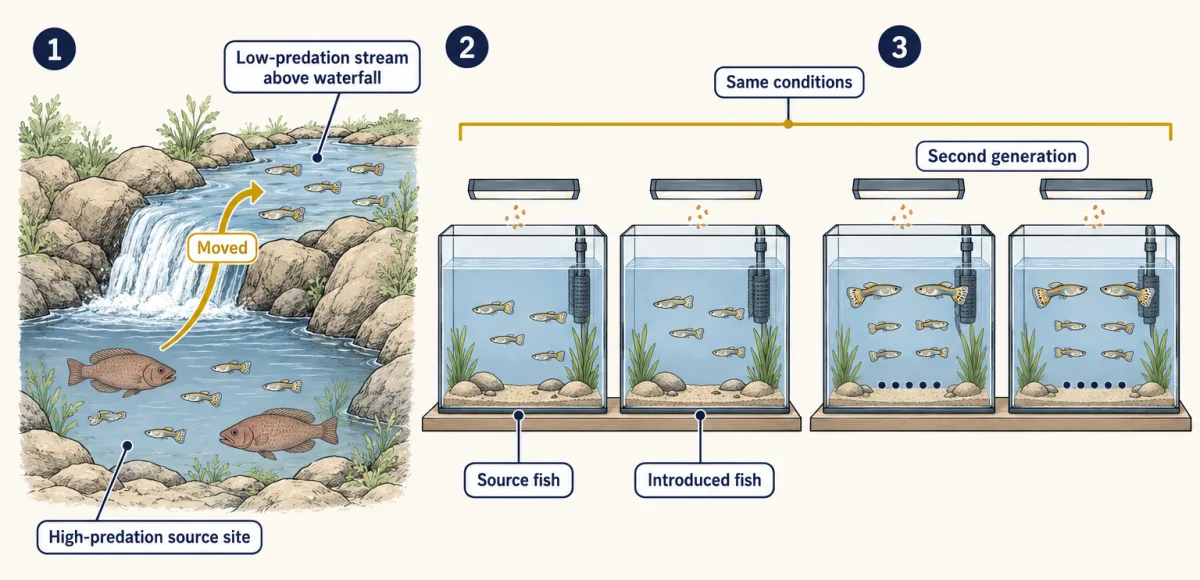
That shows a genetic basis for the difference, not its cause. Moving fish above a waterfall changes predation, and it may also change population density and food supply. To link the change to predation, compare several high- and low-predation streams, and measure density and food at each site.
The overall question, why later maturation spread where predators are few, is ultimate: it asks about adaptive significance and history. How a guppy’s body times its maturation would be a separate, proximate question.
How we measure it
Gene overexpression with an empty-vector control
Insert extra copies of a gene into a plant so that it is made in large amounts, and compare those plants with controls that went through the same procedure with a vector carrying no added gene. Differences between the two groups can then be put down to the gene rather than to the transformation process.
Epidermal impressions and light microscopy
Take an impression of a leaf surface (Hughes and colleagues pressed dental resin on the leaf, then painted clear nail varnish on the resin), peel off the varnish copy, and count the imprinted stomata in a known area under a light microscope. It gives stomatal density per square millimetre without destroying the plant.
Infrared gas analysis
Clamp an attached leaf in a small chamber and measure how much carbon dioxide and water vapour the air gains or loses as it flows past. From these you calculate the leaf's carbon assimilation, its transpiration and its stomatal conductance.
Common-environment rearing
Raise the descendants of two wild populations side by side under the same conditions, ideally for more than one generation. A difference that persists is likely to be inherited, because the environments that might have caused it directly are now the same.
Finish line
Test yourself
8 questions
Practice and MCAT-style, with explained answers.
Next · Lesson 2
Size, Scale and Surface
A 70 kg human burns far more energy than a 30 g mouse, yet each kilogram of mouse burns about seven times more. Why?
Continue →